The Role of 5-Amino-1MQ in Cellular Metabolism: NNMT Inhibition Pathways In-Vitro
21st Jun 2026
What You Need to Know About 5-Amino-1MQ
- Researchers investigate 5-Amino-1MQ to understand how blocking a specific metabolic enzyme called NNMT influences energy balance in fat and muscle cells.
- In plain terms, the compound acts like a molecular plug that stops NNMT from draining raw materials needed to make NAD+, a vital cellular fuel helper.
- Published studies in cell dishes and animal models observed higher intracellular NAD+ levels, increased SAM availability, and smaller fat cell size following exposure.
- All current findings come strictly from in-vitro cell cultures and preclinical rodent models, meaning its behaviour in people remains unestablished.
How 5-Amino-1MQ Stops the Enzyme Draining Cellular Energy
In published laboratory studies, 5-Amino-1MQ blocks an enzyme called nicotinamide N-methyltransferase (NNMT) that normally drains cellular energy reserves. By putting a brake on this enzyme, the molecule helps cultured cells keep much higher levels of NAD+, a vital coenzyme that powers mitochondrial output and cellular repair.
To understand the role of 5-Amino-1MQ in cellular metabolism: NNMT inhibition pathways in-vitro, it helps to look at how fat cells and muscle cells handle energy as they age or store excess lipids. Inside the cell, NAD+ acts like a rechargeable battery pack. It carries electrons from one reaction to another so mitochondria can turn basic nutrients into usable energy. Your cells make NAD+ through a recycling loop called the salvage pathway. This loop takes nicotinamide, a basic form of vitamin B3, and converts it back into fresh NAD+ so the energy cycle never stalls.
However, an enzyme called NNMT often gets in the way of this recycling loop. When fat tissues expand in preclinical models, NNMT levels climb sharply. NNMT grabs nicotinamide and attaches a methyl group to it, turning it into a methylated byproduct called 1-methylnicotinamide. Once nicotinamide is methylated, the cell cannot recycle it into NAD+ anymore. It simply gets flushed out of the cell. Worse still, that methyl group comes from S-adenosylmethionine (SAM), another important cellular resource. High NNMT activity therefore drains two separate pools at once: it lowers NAD+ availability and uses up methyl donors needed for normal gene expression.
5-Amino-1MQ (5-amino-1-methylquinolinium) is a small, membrane-permeable molecule built specifically to fit inside the active pocket of the NNMT enzyme. Because it shares a similar core shape with nicotinamide, it slips into the binding site and blocks NNMT from grabbing real nicotinamide molecules. Laboratory assays show that this competitive blockade stops the enzyme cold without interfering with other enzymes in the NAD+ salvage loop.
With NNMT blocked, cultured adipocytes (fat cells) and myoblasts (muscle precursor cells) stop wasting nicotinamide. Intracellular NAD+ levels rise steadily, which switches on a family of NAD+-dependent enzymes known as sirtuins, especially SIRT1. Activated SIRT1 turns on genes that favour fatty acid oxidation, glucose uptake, and mitochondrial biogenesis. Instead of slowing down and hoarding lipids, the cells shift toward higher metabolic expenditure and cleaner energy turnover. This straightforward enzyme blockade explains why researchers study 5-Amino-1MQ so closely when mapping out cellular energy expenditure and metabolic efficiency in the dish.
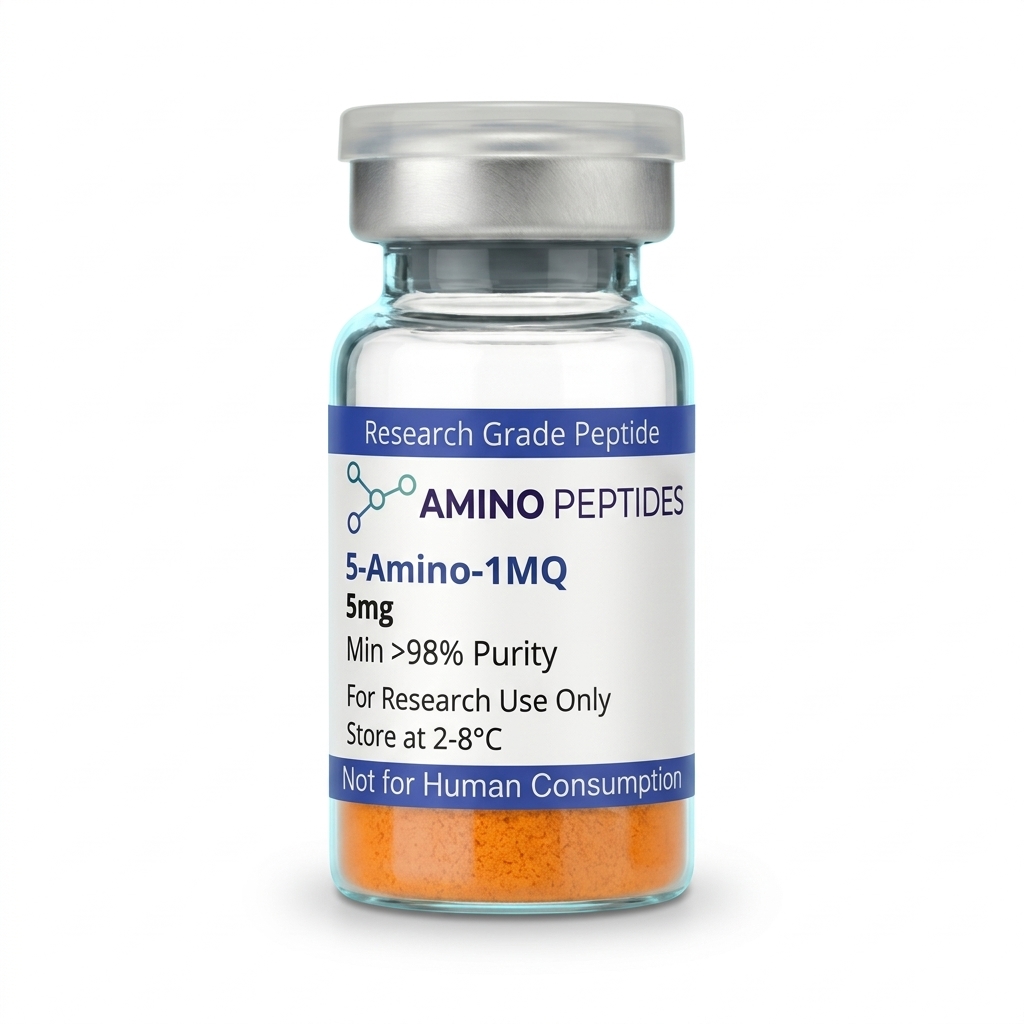
5-Amino-1MQ
From £22
Supplied as a sealed freeze-dried vial (stable 12–24 months at 2°C–8°C in a standard refrigerator).
Shop 5-Amino-1MQ →From Early NAD+ Spikes to Structural Fat Cell Changes in Vitro
When researchers add 5-Amino-1MQ to cell cultures or preclinical tissue models, the observed biological events unfold in distinct phases. Because 5-Amino-1MQ is a small quinolinium derivative with a positive charge, it crosses cell membranes quickly in vitro. Scientists do not have to wait days to see the initial biochemical shifts; the earliest changes show up within hours of applying a measured level to the culture medium.
During the first two to six hours in cultured adipocytes, direct target engagement takes place. High-performance liquid chromatography and mass spectrometry assays confirm that intracellular levels of 1-methylnicotinamide—the waste product of NNMT—drop sharply. At the same time, the ratio of SAM to S-adenosylhomocysteine (SAH) begins to recover because NNMT is no longer burning through methyl donors. By the 12-to-24-hour mark, researchers observe a measurable climb in intracellular NAD+ concentrations, often reaching 1.5 to 2 times the baseline level recorded in untreated control wells.
Between 24 and 72 hours, this extra NAD+ wakes up downstream signalling proteins. SIRT1 activity rises, which leads to the deacetylation of PGC-1alpha, a transcription cofactor that tells the cell to build and run more efficient mitochondria. During this middle window, oxygen consumption rates in the culture dish increase. Assays measuring extracellular acidification and oxygen uptake show that the cells are burning through glucose and fatty acids faster than control groups. In differentiating 3T3-L1 pre-adipocyte cultures, gene expression panels taken at 48 hours reveal a clear drop in lipogenic (fat-building) markers such as PPAR-gamma and fatty acid synthase.
Structural and morphological changes take longer to appear, typically showing up between day four and day fourteen of a laboratory protocol. In multi-day adipocyte differentiation studies, cells exposed to a steady concentration of 5-Amino-1MQ accumulate noticeably fewer and smaller lipid droplets when stained with Oil Red O. Rather than swelling into large, lipid-packed spheres, the cells stay smaller and keep higher metabolic turnover. In aged skeletal muscle satellite cell models studied over seven to ten days, blocking NNMT supports better myoblast proliferation and fusion, helping stem cells form healthier myotubes in vitro. Across all of these published studies, the pattern is consistent: rapid enzyme inhibition and NAD+ preservation in the first 24 hours, followed by metabolic gene activation over two to three days, and visible structural remodelling of lipid stores or muscle fibres over one to two weeks.
Comparison of NNMT Inhibitors in Preclinical Research
| Compound | Target Site | IC50 / Potency Profile | Cell Permeability | Primary Preclinical Observation |
|---|---|---|---|---|
| 5-Amino-1MQ | Nicotinamide binding pocket | ~1.2 uM to 2.0 uM (selective) | High (active transport and passive diffusion) | Elevated intracellular NAD+ and reduced lipogenesis in cultured 3T3-L1 adipocytes |
| 1-Methylquinolinium (1MQ) | Nicotinamide binding pocket | ~1.8 uM (moderate selectivity) | Moderate | Baseline scaffold demonstrating proof-of-concept NNMT blockade in cell lysates |
| JBSNF-000088 | Nicotinamide pocket (substrate analog) | ~1.6 uM to 2.4 uM | High | Reduced 1-MNA accumulation and improved glucose handling in rodent metabolic models |
| LL320 | Bisubstrate (SAM and nicotinamide pockets) | Low nanomolar (~1.6 nM in biochemical assays) | Very low (polar amino acid tail) | High structural specificity in purified enzyme assays but limited intact-cell activity |
| Sinefungin | SAM cofactor binding site | ~3.5 uM to 15 uM (non-selective pan-methyltransferase) | Low | Broad inhibition across multiple cellular methyltransferases with high off-target effects |
Pairing 5-Amino-1MQ with Complementary Metabolic and Signalling Peptides
In laboratory research, scientists rarely look at a single metabolic pathway in isolation. Because 5-Amino-1MQ works by plugging the leak in the NAD+ salvage pathway, investigators often pair it with complementary peptides that act on mitochondrial membranes, glucose transport, or local tissue recovery. Combining compounds that work on separate steps of the same metabolic chain allows researchers to see whether two distinct signals produce a stronger, cleaner response in vitro than either agent alone.
One of the most logical research pairings combines 5-Amino-1MQ with MOTS-c, a 16-amino-acid mitochondrial-derived peptide. While 5-Amino-1MQ raises cytosolic and nuclear NAD+ by blocking NNMT, MOTS-c works through the folate-methionine cycle to raise AICAR levels and activate AMPK, the cell's main energy sensor. When AMPK and SIRT1 are switched on at the same time in preclinical models, they reinforce each other: AMPK boosts NAD+ production further, and SIRT1 keeps AMPK active via LKB1 deacetylation. Studying both together gives investigators a complete look at how cultured myoblasts handle metabolic stress and fatty acid oxidation.
Another frequent combination in metabolic assays pairs 5-Amino-1MQ with AOD-9604, a modified fragment of human growth hormone (amino acids 177-191). AOD-9604 stimulates lipolysis—the breakdown of stored triglycerides into free fatty acids—by interacting with beta-3 adrenergic pathways in fat cells. However, freeing up fatty acids is only half the job; the cell still needs the mitochondrial capacity to burn them. In dual-agent laboratory setups, AOD-9604 encourages lipid release while 5-Amino-1MQ supplies the NAD+ and SIRT1 signalling required to oxidise those lipids inside the mitochondria.
Researchers exploring how metabolic stress interacts with cellular inflammation also run parallel assays using immunomodulatory peptides such as KPV and LL-37. Adipose tissue cultures under heavy lipid loads often release pro-inflammatory cytokines that slow down NAD+ recycling even further. Calming NF-kappaB signalling with KPV while blocking NNMT with 5-Amino-1MQ helps researchers separate pure metabolic effects from inflammatory interference. Similarly, when preparing multi-vial protocols in the lab, some dense sequences require diluted acetic acid for full solubility, whereas water-soluble quinolinium salts and short fragments dissolve cleanly in standard aqueous buffers or bacteriostatic reconstitution solution, making side-by-side assay preparation straightforward.
Figure: The Role of 5-Amino-1MQ in Cellular Metabolism: NNMT Inhibition Pathways In-Vitro
Reconstitution calculator
Choose a vial mass and a bacteriostatic reconstitution solution volume. The figure is the resulting concentration.
Concentration: 2.50 mg/mL
Per 0.01mL (10µL): 25.0 mcg
Open the full calculatorBacteriostatic reconstitution solutionWhy 99%+ Purity and Cold Storage Matter for 5-Amino-1MQ Vials
Whether an assay measures subtle shifts in intracellular NAD+ or tracks oxygen consumption over a ten-day differentiation timeline, the reliability of the data depends heavily on the purity of the material in the vial. When working with 5-Amino-1MQ and complementary research peptides, small chemical impurities can easily distort delicate enzymatic readouts in vitro.
High-grade research materials should always carry a verified purity of 99% or higher, confirmed by High-Performance Liquid Chromatography (HPLC) and Mass Spectrometry (MS). During synthesis, incomplete reactions can leave behind unmethylated quinoline precursors, residual solvents, or truncated sequences. In an enzymatic assay, even a 3% or 4% impurity load can compete for receptor binding sites or trigger off-target stress responses in cultured cells. If a batch contains leftover synthesis byproducts, adipocytes in the dish might slow their growth due to basic chemical toxicity rather than true NNMT inhibition, skewing the entire experiment.
Counter-ion selection and trifluoroacetic acid (TFA) removal are just as important. Many laboratory peptides and small molecules are purified using TFA, a strong acid that clings to positively charged amine groups. If excess TFA is not stripped away through proper ion-exchange chromatography—typically replacing it with a cleaner chloride or acetate salt—the leftover acid lowers the pH of the culture medium and damages cell membranes. In sensitive myoblast or pre-adipocyte cultures, trace TFA causes unwanted cellular swelling and drops baseline mitochondrial output, masking the exact NAD+ elevation that 5-Amino-1MQ is meant to produce. Checking batch-specific Certificates of Analysis (CoA) for both HPLC purity and clean salt forms keeps these variables out of the equation.
Once a high-purity vial arrives in the laboratory, proper thermal storage protects its molecular structure. In its lyophilised (freeze-dried) powder state, 5-Amino-1MQ is relatively stable away from light and moisture, but keeping vials refrigerated between 2°C and 8°C slows down oxidative degradation over months of storage. After adding bacteriostatic reconstitution solution to dissolve the compound for an active study, keeping the solution strictly at 2°C to 8°C and avoiding repeated freeze-thaw cycles prevents hydrolysis and aggregation, ensuring the last drop drawn from the vial performs identically to the first.
Frequently Asked Questions
Why is the role of 5-Amino-1MQ in cellular metabolism studied so heavily in laboratory models?
Researchers investigate 5-Amino-1MQ because it blocks nicotinamide N-methyltransferase (NNMT), an enzyme that slows down cellular energy usage. In published studies using isolated fat cells, blocking this enzyme preserves vital NAD+ reserves and activates sirtuin signalling pathways. This helps scientists analyse how cells regulate energy output and metabolic efficiency in-vitro.
What timeline do published studies follow when observing NNMT inhibition pathways in-vitro?
In laboratory models, measurable changes in cellular NAD+ concentration typically appear within twenty-four to forty-eight hours of exposure. Extended preclinical models observing fat cell size and metabolic gene expression generally run from ten to twenty-one days. These controlled timeframes allow researchers to characterise both immediate enzymatic shifts and longer-term cellular adaptation.
Can 5-Amino-1MQ be combined with NAD+ precursors in laboratory research protocols?
Yes, researchers frequently pair 5-Amino-1MQ with NAD+ precursors or metabolic peptides in multi-pathway cell assays. However, combining an NNMT blocker with direct NAD+ boosters can saturate cellular pathways if the protocol ratio is not carefully adjusted. Scientists must optimise each measured level separately to observe clear, accurate metabolic data.
How do laboratories verify 5-Amino-1MQ purity and manage cold storage?
Research facilities verify raw 5-Amino-1MQ purity of ninety-eight percent or higher using high-performance liquid chromatography and mass spectrometry. Lyophilised powder remains stable at minus twenty degrees Celsius for long-term storage. Once mixed with sterile laboratory solvent or bacteriostatic reconstitution solution, the liquid requires refrigeration at four degrees Celsius to prevent degradation.
Bibliography
- Neelakantan H, Vance V, Wetzel MD, et al. Selective and membrane-permeable small molecule inhibitors of nicotinamide N-methyltransferase reverse high fat diet-induced obesity in mice. Biochem Pharmacol. 2018;147:141-152. View published research
- Neelakantan H, Brightwell CR, Graber TG, et al. Small molecule nicotinamide N-methyltransferase inhibitor activates senescent muscle stem cells and improves regenerability of aged skeletal muscle. Biochem Pharmacol. 2019;163:481-492. View published research
- Kraus D, Yang Q, Kong D, et al. Nicotinamide N-methyltransferase knockdown protects against diet-induced obesity. Nature. 2014;508(7495):258-262. View published research
- Pissios P. Nicotinamide N-Methyltransferase: More Than a Vitamin B3 Clearance Enzyme. Trends Endocrinol Metab. 2017;28(5):340-353. View published research
- Babault N, Allali-Hassani A, Li F, et al. Discovery of Bisubstrate Inhibitors of Nicotinamide N-Methyltransferase (NNMT). J Med Chem. 2018;61(4):1541-1551. View published research
⚠️ Research Use Only Disclaimer: All peptides and compounds are sold strictly for in-vitro laboratory research purposes only. Not intended for human or veterinary use, not a dietary supplement, and not approved to diagnose, treat, cure, or prevent any disease or condition. For use by qualified researchers in suitably equipped laboratory environments only. Amino Peptides Ltd operates in full compliance with UK MHRA regulations and applicable EU research chemical guidelines.